
Research
Bacterial Growth
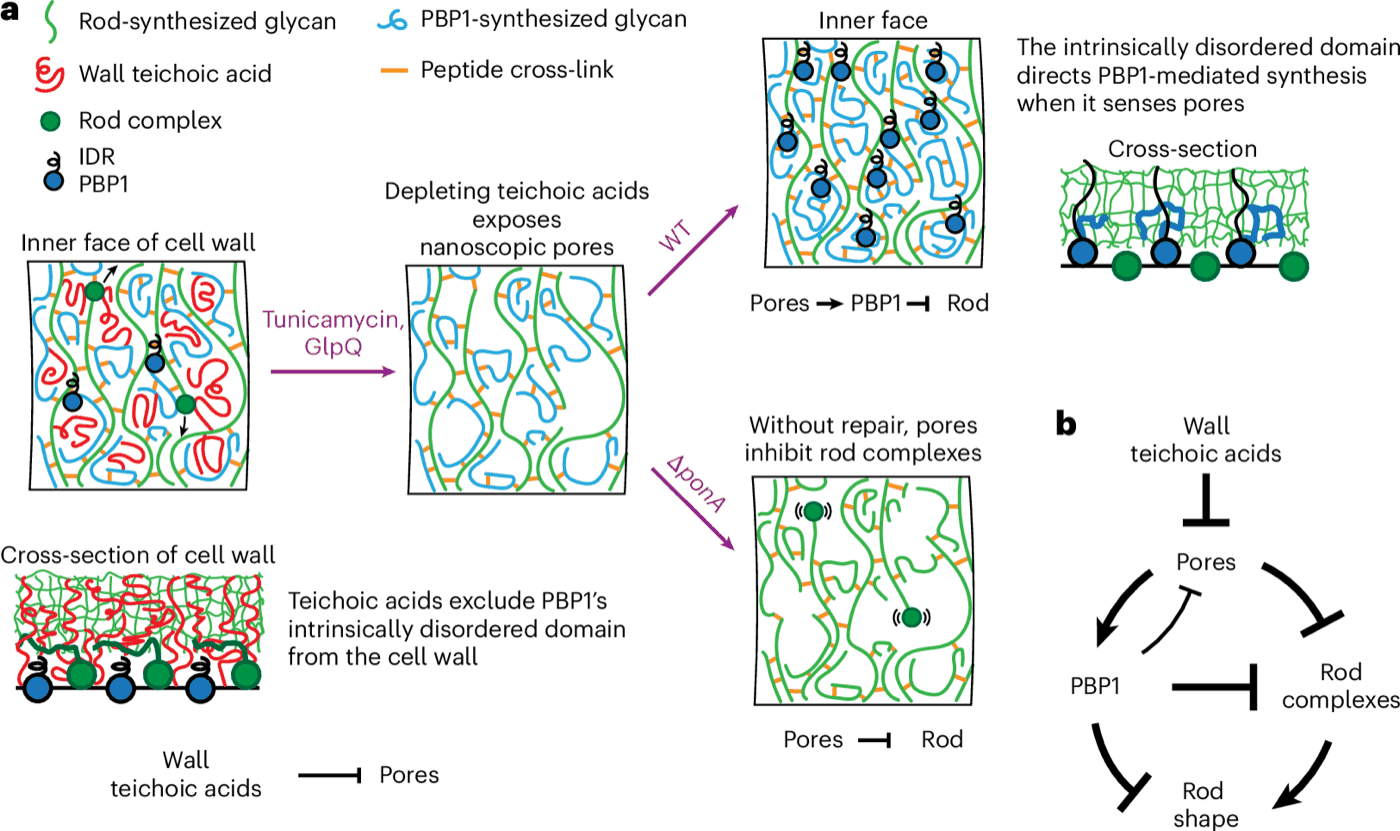
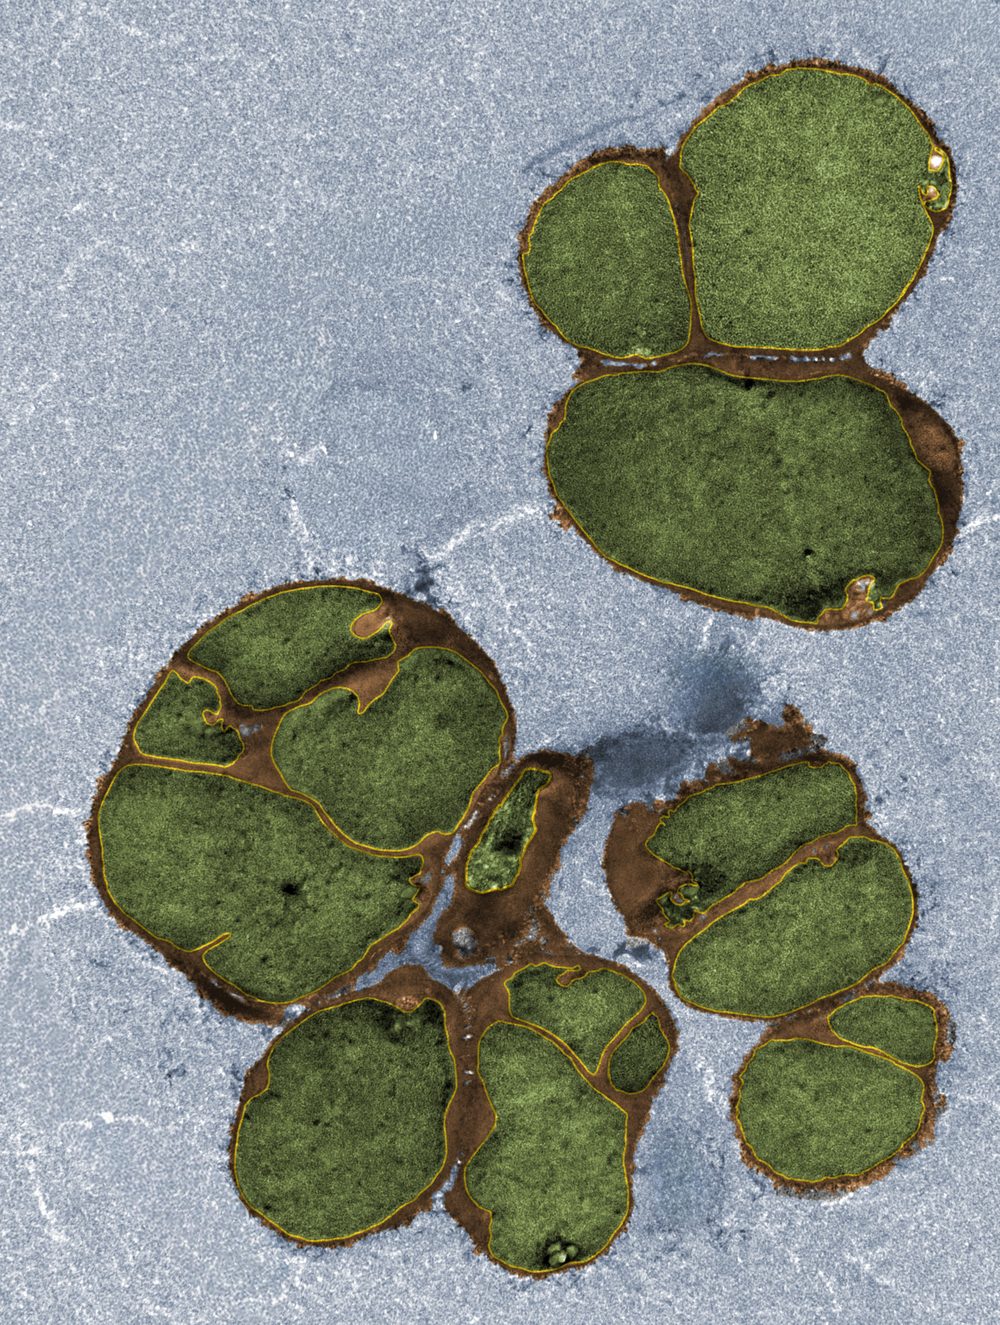
The bacterial cell wall is an essential polymeric exoskeleton that both prevents bacterial lysis and is targeted by our best frontline antibiotics. Our recent work revealed the fundamental role of wall teichoic acids, an understudied cell wall constituent of Gram-positive bacteria, in regulating both the synthesis and degradation of the primary load-bearing cell wall component: peptidoglycan. We are now leveraging these discoveries to explore the mechanistic basis of cell wall homeostasis, both with and without wall teichoic acids.
Read the paper in Nature Microbiology, or check out this research briefing for a general-audience explainer.
Budding yeast cell size control
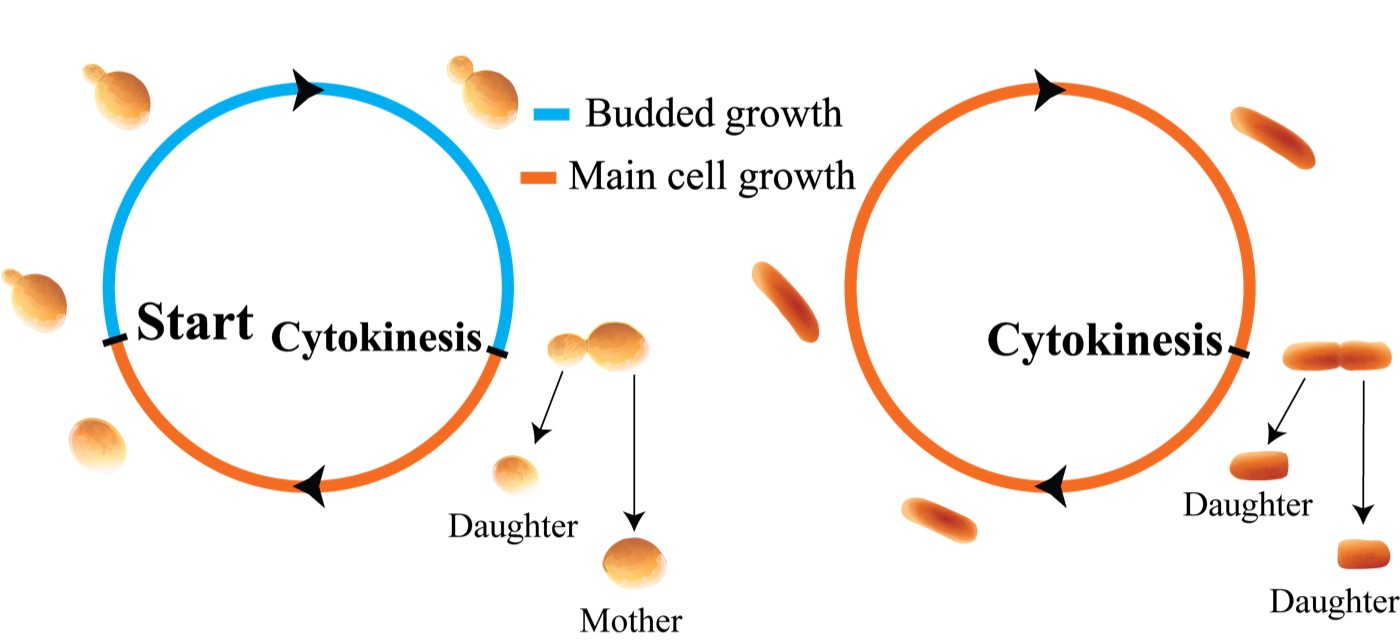
My doctoral work furthered our understanding of the mechanism and physiological consequences of cell size control in the microbe Saccharomyces cerevisiae (budding yeast), culminating in three first author publications. Cells from all domains of life regulate their size by coupling their growth and division, however, our understanding of the mechanistic origin of cell size control remains very limited.
Firstly, I used theory and simulations to study how experimentally observed cell size correlations might discriminate between two phenomenological (non-mechanistic) models of size regulation: inhibitor dilution, and initiator accumulation. We modeled asymmetrically dividing, budding cells (e.g., budding yeast) and symmetrically dividing, bacterial cells (e.g., E. coli), finding that in bacterial cells, an inhibitor dilution model did not robustly reproduce experimentally observed cell size correlations, thereby favoring an initiator accumulation model. Additionally, I discovered a model-independent constraint that symmetrically dividing, budding cells are unable to effectively regulate their size, motivating a novel hypothesis for the evolutionary origin of asymmetric division in budding yeast.
Secondly, I used experimental microbiology to test a widely supported hypothesis for size control in budding yeast. It was believed that linear, rather than exponential, accumulation of the transcriptional inhibitor Whi5 coordinates cell size with passage through the cell cycle transition “Start”. To test this model, I constructed an inducible expression system to make the Whi5 concentration independent of cell size. At a level of Whi5 expression matching WT cells, the size distributions of our inducible strains were indistinguishable from WT cells. I verified this by microscopy using a computational pipeline I developed. The Whi5 dilution model predicts that this perturbation will cause a significant increase in the spread in cell size. I observed no such increase, demonstrating that the dynamics of Whi5 expression are not the fundamental origin of size control in this organism, as previously thought. I also perturbed the expression of Cln3, an activator of Start, disproving another previously proposed model of cell size control based on the Cln3 5’ UTR.
Thirdly, I modeled the population growth rate in asymmetrically dividing cells using theory and simulations. I discovered that asymmetric cell division can enhance an organism’s growth rate in a manner that depends on cell size control, a behavior not previously observed in symmetrically dividing cells. I also disproved a prior prediction that the epigenetic inheritance of cell division times will enhance the population growth rate, showing instead that epigenetically inherited division times can arise as an intuitive consequence of cell size control in asymmetrically dividing cells.
My graduate research combined experimental and theoretical techniques to yield novel insights on outstanding questions in cell size control. My interdisciplinary research motivated a novel, testable hypothesis for the evolutionary origin of asymmetric division in budding yeast, refuted a widely supported model for the fundamental origin of size control in budding yeast, and deepened our understanding of the impact of cell shape and size control on the population growth rate. In each case, my work furthered our understanding of cell physiology beyond the narrow paradigm of symmetrically dividing, non-budding cells.
The BEC-BCS Crossover
This essay on the crossover between the Bose-Einstein Condensate and Bardeen-Cooper-Schrieffer states of matter was part of my assessment for Part III of the mathematical tripos at Cambridge. If you’re interested to see an unpublished literature review from several years ago, look no further! Part III Essay.